New clues on Norway spruce reproduction


New clues on Norway spruce reproduction
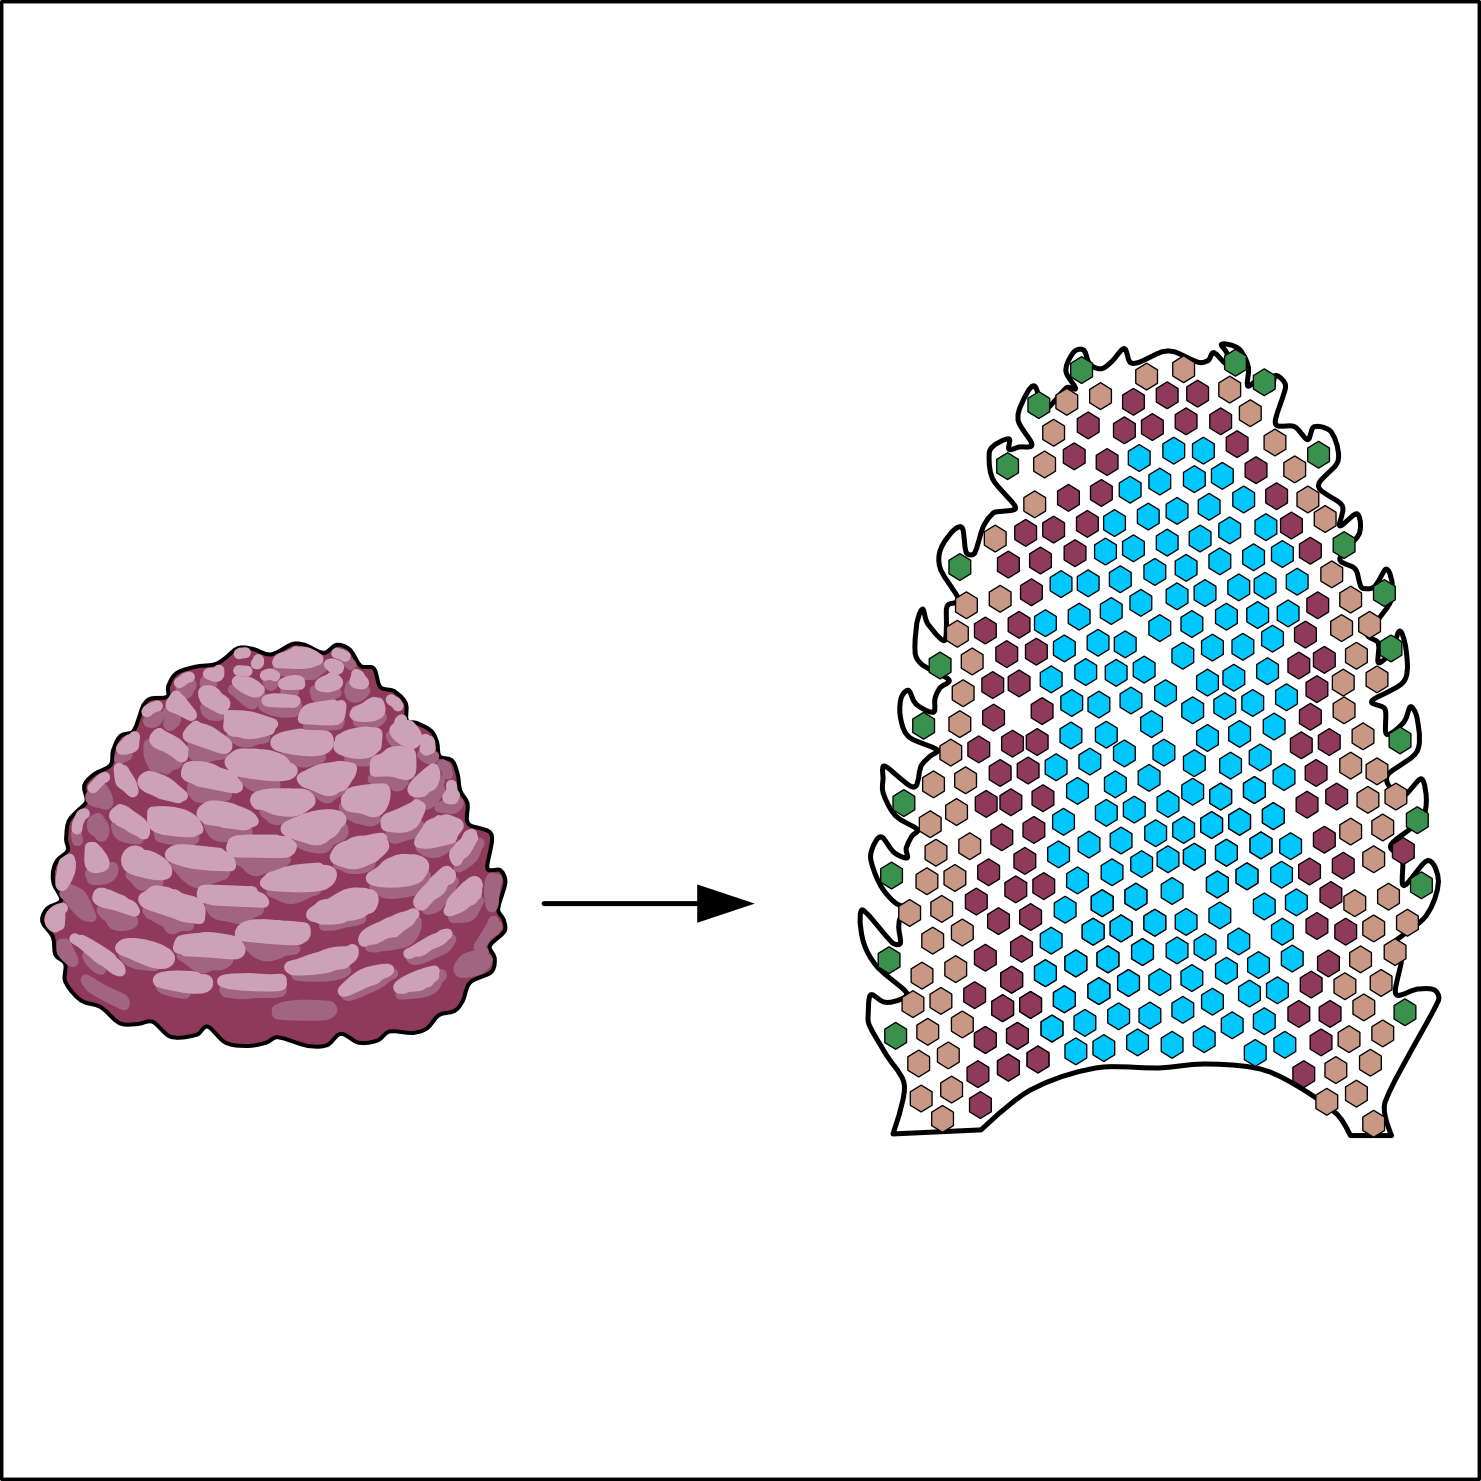
Norway spruce (Picea abies) spends its first 25 years or so of its life as a juvenile, and after that only reproduce ever 3 to 5 years. Not surprising, researchers wanted to know more about which genes are involved in the transition towards cone and seed production. Knowing this will potentially help with speeding up breeding new varieties, which for example are better suited to the changing climate. But being a slow reproducing tree with a complex genome makes this all in all complex.

Now Swedish researchers have found a way to gain insights in this tree transitioning from vegetative organ development towards cone development. Key to this was the development of a technique they called spatial transcriptomics. Spatial transcriptomics basically looks at the gene activity of small (in this case they got a 55µm resolution, and a 1µm is 0.001mm) sections or cubes across a tissue. From this the researchers can then place on a map of the tissue so they can see exactly in which bit of the tissue which genes are active.

Zooming in

Doing this allowed the researchers to distinguish which genes are active in the inner pith vs the vascular tissue and the outer developing lateral organs. Giving them a colourful map of all the different cell types in the tissue sample they analysed.

In this case, as the researchers wanted to know more about what genes are involved in the transition from vegetative tissue towards reproductive cone tissue, the researchers looked at developing shoot tissue at three different time points during this transition.

After having done the initial spatial transcriptomics and analysis the researchers zoomed in on a gene known from earlier studies to be involved in the transition from vegetative to reproductive cone, the gene activator SPL1. And as it is known that SPL1 is negatively controlled by miR156 and miR529, the researchers included these as well.

Creating a genetic model

First thing they did was checking the gene activity of these genes. Finding that the gene activity of SPL1 is low in vegetative tissue but high in the developing cones. For miR156 and miR529 the opposite was found.

Next, the researchers looked at the spatial transcriptomics data to find the genes whose activity correlated with the gene activity of SPL1. Identifying two gene activators, DAL14 and the up till now unknown DAL55. Both DAL14 and DAL55 were active when SPL1 was active and showed low activity when SPL1 activity was low. This suggests that DAL14 and DAL55 could be activated by SPL1, and that both genes are important for cone development

The researchers tested if SPL1 could potentially activate DAL14 and DAL55. Which it could. But that is how far the researchers were able to dive into the molecular mechanism of how Norway spruce is regulating its transition from vegetative towards reproductive cone tissue.

Next up will not only be to expand the genetic model of cone production initiation but also trying to find out what triggers the transition from vegetative towards cone tissue. So, what inhibits miR156 and miR529 activity. This especially might help with attempts to speed up breeding novel varieties that might be better suited to the changing climate.

Literature

Saarenpää et al., Norway spruce spatiotemporal programs of conifer reproductive development, Cell (2026), https://doi.org/10.1016/j.cell.2026.08.033

Thanks for reading.
If you like what you read, support me with on of the following actions

Follow me on LinkedIn or BlueSky
Share it with a friend or co-worker
Singing up to my newsletter so my next blog lands directly in your inbox

Nieuwe aanwijzingen voor fijnspar reproductie


Nieuwe aanwijzingen voor fijnspar reproductie

De jeugd van fijnsparren (Picea abies) duurt 25 jaar, en zelfs daarna produceert de boom maar eens in de 3 tot 5 jaar zaden. Niet verwonderlijk dat onderzoekers meer wilde weten over welke genen betrokken zijn bij de overgang naar kegel en zaden productie. Dat kan namelijk helpen met de veredeling van nieuwe varianten die bijvoorbeeld beter bestand zijn tegen het veranderende klimaat. Maar dit uitzoekenen voor een langzaam reproducerende boom met ook nog eens een complex genoom is alles bij elkaar simpel gezegd complex.

Maar nu hebben Zweedse onderzoekers een manier gevonden om inzichten te verkrijgen in de overgang van vegetatieve ontwikkeling naar kegel ontwikkeling van deze boom. De sleutel hiertoe lag in de ontwikkeling van een techniek genaamd spatiale transcriptomics. Spatiale transcriptomics kijkt in principe naar de gen activiteit van kleine (in dit geval keken ze op 55µm resolutie; 1 µm is 0,001 mm) delen of blokjes van een weefsel. Deze gen activiteit plaatsen de onderzoekers vervolgens op een kaart van het weefsel, zodat ze precies kunnen zien in welk gedeelte van een weefsel de genen actief zijn.

In zoomen

Hierdoor konden de onderzoekers onderscheid hoe actief een gen is in het binnenste van de stengel vs de vaatbundels, en de buitenste ontwikkelende organen. Dit gaf de onderzoekers een kleurrijke kaart van de verschillende celtypen in het weefsel dat ze analyseerde.

In dit geval, omdat de onderzoekers meer wilde weten over de genen die betrokken zijn in de overgang van vegetatieve weefsel naar reproducerend kegel weefsel, keken de onderzoekers naar het ontwikkelende stengelweefsel op drie verschillende momenten van deze overgang.

Na de spatiale transcriptomics en analyse daarvan gedaan te hebben, zoomde de onderzoekers in op een gen waarvan bekend is dat het betrokken is in deze overgang, de gen activator SPL1. En omdat het bekend is dat miR156 en miR529 SLP1 negatief reguleren, namen de onderzoekers deze ook mee in hun verdere analyse.

Een genetisch model creëren

Het eerste wat de onderzoekers deden was de gen activiteit van deze genen nagaan. Hierbij vonden ze dat de activiteit van SPL1 laag is in vegetatief weefsel, maar hoog is in de ontwikkelende kegels. Voor miR156 en miR529 was het tegenover gestelede het geval.

Vervolgens keken de onderzoekers at de spatiale transcriptomics data om de genen te vinden wiens activiteit correleerde met dat of SPL1. Dit resulteerde in de identificatie van twee gen activators, DAL14 en de tot nu toe onbekende DAL55. Zowel DAL14 als DAL55 zijn actief op het moment dat SPL1 ook actief is, en hadden lage activiteit wanneer SPL1 lage activiteit had. Dit suggereert dat DAL14 en DAL55 door SPL1 geactiveerd kunnen worden, en dat beide genen belangrijk voor kegel ontwikkeling zijn.

De onderzoekers gingen na of SPL1 DAL14 en DAL55 gen activiteit kon activeren, wat het kon. Maar dit is tot hoe ver de onderzoekers tot nu toe het mechanisme konden ontrafelen van hoe fijnspar z’n overgang van vegetatieve weefsel naar kegel weefsel reguleert.

Voor de toekomst is niet alleen belangrijk om het moleculaire model van de initiatie van kegel ontwikkeling uit te breiden, maar ook om de uit te vinden van de transitie van vegetatief naar kegel weefsel in gang zet. Dus wat stopt de activiteit van miR156 en miR529. Dit kan vooral helpen met pogingen om de veredeling van nieuwe fijnspar varianten die beter toegepast zijn voor het veranderende klimaat te versnellen.

Literatuur

Saarenpää et al., Norway spruce spatiotemporal programs of conifer reproductive development, Cell (2026), https://doi.org/10.1016/j.cell.2026.08.033


Bedankt voor het lezen
Vond je het interessant, overweeg dan een van de volgende acties

Volg me op LinkedIn of BlueSky
Stuur het door aan een vriend of collega

Abonnneer je op m’n nieuwsletter zodat de volgende automatisch in je inbox verschijnt.

Negative regulation of a still to be discovered hormone


Negative regulation of a still to be discovered hormone

Often the messenger is discovered first and followed by the messenger recognising receptor and signalling pathway that is activated in response to this messenger. So, it appeared to be for karrakin, a messenger molecule in plant derived smoke, that activates responses in fire-adapted plants, like seed germination. Only after identifying the karrakin receptor, KAI2, in those fire-adapted plants it quickly became clear that those receptors could also be found in other plants.

Plants like Arabidopsis respond to karrakins by adjusting their growth and development. The processing of karrakin perception happens in a similar manner as the perception of the hormone strigolactone but using different protein family members and regulating a different set of genes.

This all was found out with help of karrakins. But it was the discovery that plants without KAI2 show the opposite phenotype to plants treated with karrakins, that made scientist to suggest that plants are producing karrakin-like (KL) molecules.

Negative feedback

Up till now the majority of the studies focussed on the response to karrakin(-like) and how plants regulate this. But hormone response is often held in check by negative feedback loops. Now a new study by a group of international researchers focused on this negative feedback loop.

They found a likely candidate to be part of this negative feedback loop in DLK2. DLK2 is a protein that looks a lot like KAI2 but without the ability to directly interact with the same proteins KAI2 interacts with. So, the question was how does DLK2 work.

First the researchers confirmed that DLK2 was indeed negatively regulating karrakin(-like) response. Having done that, they came up with two hypotheses. The first was that DLK2 breaks down KL molecules. The second was that DLK2 interfered with the interaction of KAI2 with its target protein, SMAX1, whose breakdown by KAI2 results in activating KL-response genes.

Hypothesis testing

Having no way of testing if DLK2 breaks down a molecule whose identity is not known, the researchers had to find a way around that. They did three tests. The first was to find out if DLK2 needs to be in the nucleus to do its job, because KAI2 and SMAX1 both need to be there to do their job.

Having created DLK2 proteins that were either localised in the nucleus or outside the nucleus. The researchers then combined those with a reporter system that is activated by SMAX1. This showed that DLK2 localised in the nucleus and localised outside the nucleus both prevented SMAX1 breakdown. Suggesting that DLK2 doesn’t need to be in the nucleus to do its job. Putting one strike against hypothesis number two.

Subsequently the researchers tested if DLK2 when in the vicinity of KAI2 and SMAX1 interfered with their interaction. Using again a reporter that lighted up when KAI2 and SMAX1 interacted the researchers noticed that with karrakin present DLK2 was not able to reduce the signal of the reporter. Suggesting that DLK2 was not interfering with the interaction between KAI2 and SMAX1. Putting a second strike against hypothesis number 2.

Breaking down karrakin like molecules

Lastly the researchers tested if DLK2 could break down karrakin-like molecules. Testing with a variety of molecules the researchers noticed that DLK2 broke down a KL-like molecule called Yoshimulactone Green, but not it closely resembling desmethyl Yoshimulactone Green. Suggesting that DLK2 has KL breakdown activity needed for the support of hypothesis number one.

Al together, this study shows that DLK2 functions as a negative regulator of karrakin-like signalling. It does this by breaking down karrakin-like molecules so they can no longer activate karrakin-like signalling. But that is not all this study shows. It also shows that even if the substrate or messenger molecule is not known, there is still a lot to be found out about how the plant regulates responding to that messenger molecule.

Literature

Q. Li, et al., 2026, Negative feedback regulation of karrikin signaling in Arabidopsis thaliana by an antagonistic paralog of karrikin receptors, Proc. Natl. Acad. Sci. U.S.A. 123 (37) e2525145123, https://doi.org/10.1073/pnas.2525145123.


Thanks for reading.
If you like what you read, support me with on of the following actions

Follow me on LinkedIn or BlueSky
Share it with a friend or co-worker
Singing up to my newsletter so my next blog lands directly in your inbox

Negatieve regulatie van een nog te ontdekken hormoon


Negatieve regulatie van een nog te ontdekken hormoon

Vaak is het zo dat de boodschapper wordt ontdekt voor de ontdekking van de boodschapper herkennende receptor en de actie die op de detectie van de boodschapper volgt. Zo leek het te zijn voor karrakin, een boodschapper molecuul in van planten afkomstige rook, die in vuur-aangepaste planten voor specifieke reacties zorgt, zoals ontkieming van zaden. Alleen bleek al snel na de ontdekking van de karrakin receptor, KAI2, in die vuur-aangepaste planten, dat die receptor ook in andere planten aanwezig was.

Planten zoals Arabidopsis passen hun groei en ontwikkeling aan na waarneming van karrakin. De verwerking van de waarneming van karrakin gebeurt op een vergelijkbare manier als de verwerking van de waarneming van het hormoon strigolactone, maar het gebruikt andere leden van dezelfde eiwit familie en reguleert een ander genen set.

Dit alles was ontdekt met behulp van karrakins. Maar het was de ontdekking dat planten zonder KAI2 precies het tegenovergestelde fenotype van dat van planten behandelt met karrakins vertoonde dat onderzoekers deed suggereren dat planten op karrakin gelijkende (KL) moleculen produceren.

Negatieve feedback

Tot nu toe focuste de meeste studies op de reactie op karrakins en hoe planten dit reguleren. Maar hormoon reacties worden vaak gecontroleerd met behulp van negatieve feedback loops. Een nieuwe studie door een internationale groep van wetenschappers focust zich op die negatieve feedback loop.

De onderzoekers vonden in DLK2 een mogelijke kandidaat voor deze negatieve feedback loop. DLK2 is een eiwit dat veel op KAI2 lijkt, maar dan zonder de mogelijkheid om de interactie aan te gaan met dezelfde eiwitten. Dus de vraag was, hoe gaat DLK2 te werk.

Het eerste wat de onderzoekers deden is bevestigen dat DLK2 inderdaad betrokken was in de negatieve feedback loop. Na dit gedaan te hebben kwamen de onderzoekers met twee hypothesen. De eerste was dat DLK2 KL moleculen afbreekt. De tweede was dat DLK2 de interactie verstoord tussen KAI2 en z’n doel eiwit, SMAX1 wiens afbraak resulteert in de activatie van KL-reactie genen.

Hypothesis testen

Zonder een manier te hebben om direct te testen of DLK2 een nog onbekend molecuul afbreekt, moesten de onderzoekers een andere manier vinden om de hypothesen te testen. Ze deden drie testen. De eerste was om uit te vinden of DLK2 in de nucleus moet zijn om z’n werk te doen, omdat KAI2 en SMAX1 allebei in de nucleus moeten zijn voor hun werk.

De onderzoekers creëerde DLK2 eiwitten die of in de nucleus of niet in de nucleus zaten. Die combineerde de onderzoekers vervolgens met een reporter systeem dat geactiveerd wordt door SMAX1. Dit liet zien dat zowel DLK2 gelokaliseerd in als buiten de nucleus afbraak van SMAX1 voorkomt. Dit suggereert dat DLK2 niet in de nucleus hoeft te zijn om z’n werk te doen. En geeft een minpunt aan hypothese nummer twee.

Vervolgens testen de onderzoekers of in DLK2 in de nabijheid van KAI2 en SMAX1 de interactie tussen die twee verstoorde. Dit deden ze met behulp van een reporter die oplichtte wanneer KAI2 en SMAX1 interacteerde. Het viel de onderzoekers op dat met karrakin aanwezig DLK2 niet in staat was om het signaal van de reporter te verminderen. Dit suggereert dat DLK2 de reactie tussen KAI2 en SMAX1 niet verstoord. En een tweede minpunt voor hypothese nummer twee.

Afbraak van kerrakin gelijkende moleculen

Als laatste testte de onderzoekers of DLK2 op karrakin gelijkende moleculen kon afbreken. De onderzoekers testte verschillende moleculen en zagen zo dat DLK2 een op KL-lijkend molecuul genaamd Yoshimulactone Green afbrak maar niet het vergelijkbare molecuul desmethyl Yoshimulactone Green. Dit suggereert dat DLK2 de voor hypothese nummer een benodigde KL afbraak activiteit bezit.

Samengevat laat deze studie zien dat DLK2 functioneert als een negatieve regulator van karrakin gelijkende signalering. Het doet dit door op karrakin gelijkende moleculen af te breken. De studie laat ook zien dat zelfs al is het substraat of boodschapper molecuul onbekend, er nog steeds een hoop te ontdekken is of hoe de plant de reactie op dat onbekende molecuul reguleert.

Literatuur

Q. Li, et al., 2026, Negative feedback regulation of karrikin signaling in Arabidopsis thaliana by an antagonistic paralog of karrikin receptors, Proc. Natl. Acad. Sci. U.S.A. 123 (37) e2525145123, https://doi.org/10.1073/pnas.2525145123.


Bedankt voor het lezen
Vond je het interessant, overweeg dan een van de volgende acties

Volg me op LinkedIn of BlueSky
Stuur het door aan een vriend of collega

Abonnneer je op m’n nieuwsletter zodat de volgende automatisch in je inbox verschijnt.